mtDNA · Maternal lineage

G2B1

mtDNA Haplogroup G2B1

A reference profile for one lineage branch. Shared haplogroups do not establish a family relationship or cultural identity.

Reference profile

Branch background

Historical context for mtDNA lineage branch G2B1

Origins and Evolution

mtDNA haplogroup G2B1 is a downstream branch of the broader G2/G haplogroup family. It likely emerged in Northeast Asia during the early Holocene (on the order of ~8 thousand years ago), a period of climatic amelioration and population reorganization after the Last Glacial Maximum. The coalescence time for G2B1 is younger than its parent clade G2B (estimated ~10 kya), consistent with a local differentiation event within populations inhabiting the Japanese archipelago, the Russian Far East, and adjacent Siberian regions. As with many mtDNA lineages, G2B1's phylogeography reflects both deep Paleolithic/early Holocene settlement patterns and later population movements and contacts.

Subclades

G2B1 exhibits internal structure detectable with high-resolution mtDNA sequencing; however, the fine-scale nomenclature and number of named downstream subclades vary between studies. Some population surveys that include full mitogenomes report further branches within G2B1 consistent with localized diversification (for example, geographically restricted lineages in Hokkaido/Ainu or among particular Siberian groups). Because mitochondrial phylogenies are continually refined with new mitogenomes, researchers should consult up-to-date phylogenetic trees (e.g., Phylotree, GenBank mitogenomes) for the most current subclade labels and their distributions.

Geographical Distribution

G2B1 shows a clear Northeast Asian focus. It is most frequent and diverse in Japan — including elevated representation among Ainu and some Ryukyuan groups — and in parts of eastern Siberia. Moderate occurrences are reported in Koreans and northeastern Han Chinese, and it reaches low to moderate frequencies in Mongolic populations (e.g., Buryat) and other adjacent Central and North Asian communities. Very low-frequency and often isolated occurrences have been documented in circumpolar groups and sporadically in the Americas; these are typically interpreted as the result of recent Siberian–circumpolar gene flow or rare long-distance movements rather than a dominant founding lineage for New World populations.

Historical and Cultural Significance

The distribution of G2B1 is informative for reconstructing Holocene population dynamics in Northeast Asia. Its presence in Jomon-associated skeletal series and modern Ainu supports a role in the maternal heritage of long-term inhabitants of the Japanese archipelago. In Siberia and the Russian Far East, G2B1 aligns with lineages typical of Holocene hunter-gatherer and later circumpolar groups, indicating continuity as well as regional exchanges along coastal and inland routes. In populations of the Korean peninsula and northeastern China, G2B1 likely reflects admixture between local East Asian agricultural/forager groups and northern forager-derived gene pools.

Archaeologically, G2B1 is often discussed in relation to the Jomon cultural complex (as a primary association), and to later coastal cultures of the Okhotsk and other northern maritime traditions where continuity of maternal lineages can be observed. It is less strongly tied to Bronze Age steppe movements and more indicative of East Asian/Amur–Okhotsk–Japanese regional demographic histories.

Conclusion

G2B1 is a Northeast Asian maternal lineage that encapsulates aspects of early Holocene differentiation and subsequent regional demography in Japan and Siberia. While not among the most globally widespread mtDNA haplogroups, its geographic concentration and occasional deep splits make it a useful marker for studies of Jomon ancestry, Siberian hunter-gatherer continuity, and the complex peopling history of Northeast Asia and adjacent circumpolar zones. Continued mitogenome sampling, especially from ancient remains, will refine subclade structure and timing and clarify low-frequency occurrences outside the core range.

Key Points

  • Origins and Evolution
  • Subclades
  • Geographical Distribution
  • Historical and Cultural Significance
  • Conclusion
Reference profile

Tree & Relationships

Phylogenetic context and subclades

Evolution Path

Follow the recorded parent branches toward G2B1. Dates are estimates and can change as reference data is revised.

Steps Haplogroup Age Estimate Archaeology Era Time Passed Immediate Descendants Tested Modern Descendants Ancient Connections
1 G2B1 Current ~8,000 years ago Neolithic 8,000 years 1 5 0
2 G2B ~10,000 years ago Neolithic 10,000 years 2 6 6
3 G2 ~20,000 years ago Mesolithic 20,000 years 2 49 10
4 G ~35,000 years ago Paleolithic 35,000 years 4 382 3
5 M12'G - - - 2 383 0
6 M ~60,000 years ago Paleolithic 60,000 years 42 2,671 41
7 L3 ~70,000 years ago Paleolithic 70,000 years 7 30,162 6
8 L3'4 - - - 2 30,212 0
9 L3'4'6 - - - 2 30,216 0
10 L2'3'4'6 - - - 2 31,333 0
11 L2'3'4'5'6'7 - - - 2 31,349 0
12 L1'2'3'4'5'6'7 - - - 2 31,852 0
13 L ~160,000 years ago Paleolithic 160,000 years 2 32,236 5

Siblings (1)

Other branches from the same parent haplogroup

Reference profile

Where in the World

Geographic distribution and modern presence

Recorded origin

Northeast Asia (Japan and Siberia)

Modern Distribution

The populations where mtDNA haplogroup G2B1 is found include:

  1. Japanese populations (including Ainu and some Ryukyuan groups)
  2. Koreans and northeastern Han Chinese
  3. Indigenous Siberian groups (e.g., Yakut, Evenk, Nganasan, Koryak)
  4. Mongolic and some Central Asian populations (e.g., Buryat, Mongol)
  5. Northern Tibeto-Burman and other highland East Asian groups (at low to moderate frequencies)
  6. Circumpolar communities and rare occurrences in the Americas (generally low frequency and localized)
Historical context

A branch through time

Estimated formation in a broad historical timeline. Period markers provide context and do not imply a connection with particular cultures.

  1. ~10k years ago

    Neolithic Revolution

    Agriculture begins, settled communities form

  2. ~8k years ago

    Haplogroup G2B1

    Estimated formation of this mtDNA branch; dates and locations are reference estimates.

    This branch
  3. ~5k years ago

    Bronze Age

    Metalworking, writing, and early civilizations

  4. ~3k years ago

    Iron Age

    Iron tools, expanded trade networks

  5. ~2.5k years ago

    Classical Antiquity

    Greek and Roman civilizations flourish

  6. Present

    Present Day

    Modern era

Reference profile

Archaeological context

Recorded archaeological associations for mtDNA branch G2B1

Recorded associations

These labels describe archaeological contexts recorded for reference samples linked to G2B1. An association does not establish that all carriers belonged to a culture or followed a particular migration route.

Austria_Avar Chinese Paleolithic Early Avar Khovd Bronze Age Slab Grave Culture Thai Iron Age Upper Yellow River Culture Uvurkhangai Culture Yappa Nhae
Culture assignments are based on archaeological context of ancient DNA samples and may represent regional associations during specific time periods.
Reference profile

Sample Catalog

6 subclade carriers of haplogroup G2B1 (no direct carriers in the current reference selection)

6 shown · 6 matching samples

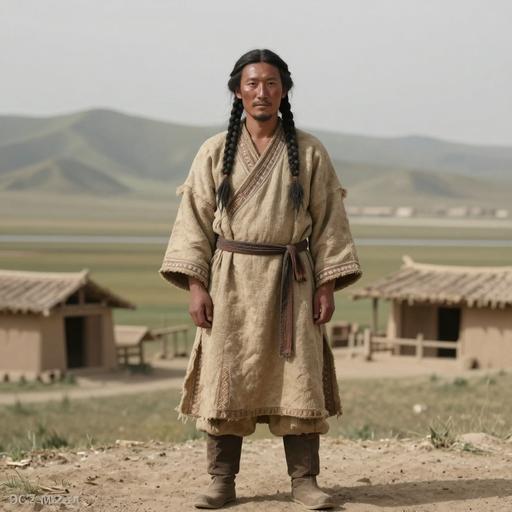
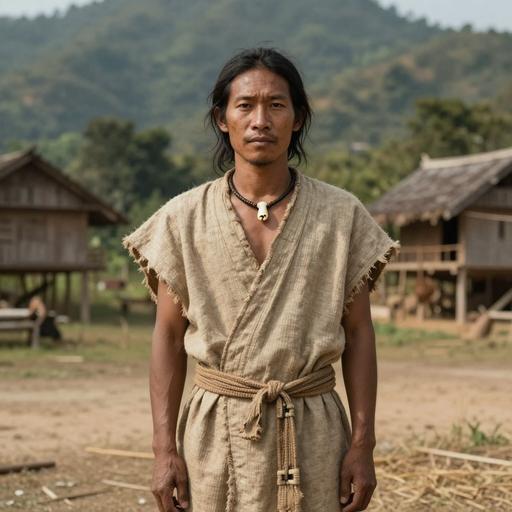
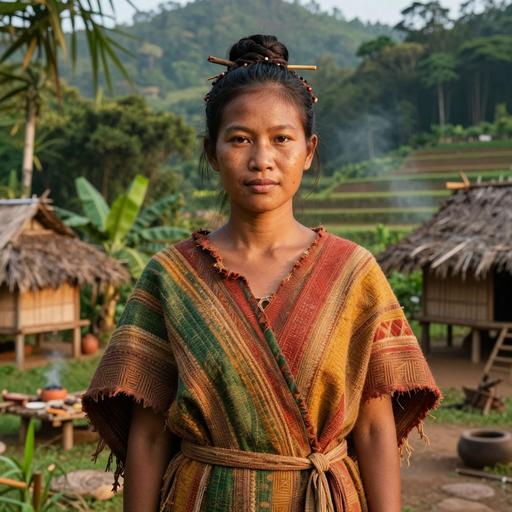
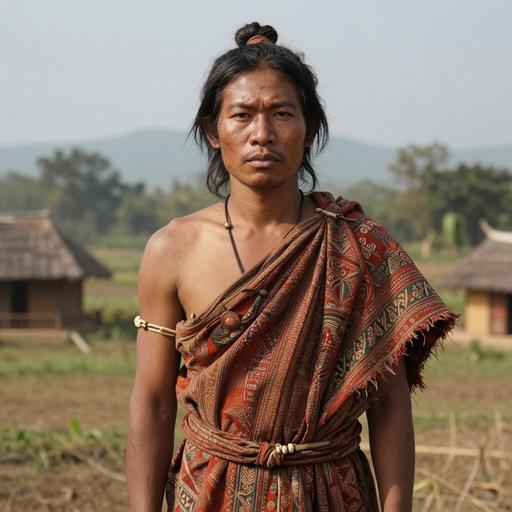
Portraits are AI-generated illustrations. Sample labels and accession IDs identify the reference records.

Portrait Sample Country Era Date Culture mtDNA Match
AI-generated illustrative portrait of Ancient Chinese Civilization individual, Qinghai province. Pingan county. Dacaozi site, China (120-248 CE)
Sample ID: DCZ-M21II
China Iron Age Upper Yellow River, China 120 CE - 248 CE Upper Yellow River Culture G2b1b Subclade
AI-generated illustrative portrait of Han individual, Qinghai province. Pingan county. Dacaozi site, China (120-248 CE)
Sample ID: DCZ-M21II
China Han Dynasty China 120 CE - 248 CE G2b1b Subclade
AI-generated illustrative portrait of IA Log Coffin individual, Yappa Nhae 2 (Mae Hong Son Province), Thailand (200-450 CE)
Sample ID: YPN018
Thailand Yappa Nhae Log Coffin Culture Iron Age 200-450 CE Yappa Nhae G2b1a Subclade
AI-generated illustrative portrait of IA Log Coffin individual, Yappa Nhae 2 (Mae Hong Son Province), Thailand (200-450 CE)
Sample ID: YPN023
Thailand Yappa Nhae Log Coffin Culture Iron Age 200-450 CE Yappa Nhae G2b1a Subclade
AI-generated illustrative portrait of IA individual, Northern Mae Hong Son. Long Long Rak, Thailand (238-376 CE)
Sample ID: Th530
Thailand Thailand IA 238-376 calCE (1756±26 BP, OxA-34838) Thai Iron Age G2b1a Subclade
AI-generated illustrative portrait of IA individual, Northern Mae Hong Son. Long Long Rak, Thailand (259-419 CE)
Sample ID: Th531
Thailand Thailand IA 259-419 calCE (1687±24 BP, OxA-34839) Thai Iron Age G2b1a Subclade
MATERNAL LINEAGE · ANCIENT DNA

Ancient lineage evidence map

Follow parent clades toward this branch and explore where ancient carriers were found.

Loading ancient observations…

Markers are archaeological find locations. A dashed connector is an uncertain, proposed geographic transition between consecutive branches supported by multiple dated observations; it is not an exact travel route, birthplace or proof of direct descent. Parent-clade samples may belong to other descendant branches. Gaps remain where evidence is insufficient. Sample dates differ from haplogroup formation dates.

Reference profile

Carrier Distribution Map

Geographic distribution of 6 ancient DNA samples (direct and subclade carriers of G2B1)

Subclade carrier
Time Period Filter
All Time Periods
Showing all samples
Reference profile

Temporal Distribution

Distribution of carriers across archaeological periods

Reference profile

Geographic Distribution

Counts by recorded sample country. These reflect the available reference selection, not population frequencies.

Reference profile

Country × Era Distribution

Compare recorded sample counts across countries and archaeological periods. Select a populated cell to inspect a sample.

Data

Data & Provenance

Source information and data quality

Last Updated 2026-02-16
Confidence Score 50/100
Coverage Low

Data Source

Classification, estimated dates and geographic context reflect the recorded reference data and may change as evidence is revised. Sample coverage is uneven; recorded locations and archaeological associations do not establish personal origin or cultural identity.

A haplogroup follows one maternal or paternal line. The branch prediction depends on which markers the DNA file contains. How our analysis works